Cell mechanics
What role do cell shape and mechanical interactions play as crypts form?
Physics · Syracuse University
Physics · Syracuse University
In Treatise of Man (1633), Discourse on the Method (1637), and Meditations (1641), René Descartes separated mind from body and laid out the bête-machine (“animal-machine”) doctrine: all non-human organisms and all biological bodies are mechanical automata, incapable of genuine learning, cognition, or agency without a rational mind directing them; even a trained animal was, for him, only a rearranged machine. Modern biology dropped the Cartesian soul but kept much of its top-down control architecture, handing the mind’s role to the central nervous system or to the genome and its “master regulator” genes, and treating the body and its material environment as passive hardware executing instructions (Nicholson 2014).
Yet across scales, matter routinely violates this hierarchy. Bacteria coordinate collective decisions through chemical quorum sensing, without a leader (Miller & Bassler 2001); developing tissues pattern through cell–matrix mechanochemical feedback (Mammoto & Ingber 2010); and disordered solids encode memories of past deformations in their own degrees of freedom (Keim et al. 2019).
Physics treats learning as a problem any adaptive material faces, constrained by how energy flows through it, how it is built, and how forces act within it. My doctoral work starts from this bottom-up view and asks how much matter can achieve through local mechanics, without a central controller. In the bacterium E. coli, I trained a model of the disordered cell wall to steer the cell away from surfaces, with no brain. In spring networks, I study why continual learning exhausts the capacity to learn, why restoring it calls for an offline, sleep-like phase, and whether sleep–wake rhythms can emerge spontaneously. In intestinal organoids, I am modeling how crypts form, using a 3D vertex model of a spheroid in a fiber-network matrix (Zhang & Schwarz 2022; Zhang et al. 2025; Ameen et al. 2026).
New here? Begin at “Start here” and follow the glowing line.
Loading the spring…
Loading physical learning…
Loading Sleep in spring networks…
Loading the interactive model…
Loading the network…
Loading feedback…
Loading self-organization…
Loading active matter…
Loading disordered matter…
Loading adaptation…
Loading the automaton…
Loading the genome…
Loading the regulator…
Loading the ecology…
Loading material-semiotic…
Can a trained cell wall help a bacterium leave a surface?
The wall itself can steer. On the first tumble after the cell is trapped at a surface, the trained model recovers 89% of the advantage of an ideal controller.
Bacterial navigation is usually modeled top-down: a chemical signaling cascade (chemotaxis; Sourjik & Wingreen 2012) acts as the cell’s brain, and the cell wall is passive hardware. This project asks whether the wall itself can steer.
We model the E. coli peptidoglycan wall as a disordered spring network and train its crosslink stiffnesses. The trained wall carries the load of a surface collision across the cell to motors on the far side. There the load destabilizes stator units, the force-generating parts of each motor, which respond to mechanical load (Lele et al. 2013; Wadhwa et al. 2019). The push becomes uneven, and the cell turns away from the trap.
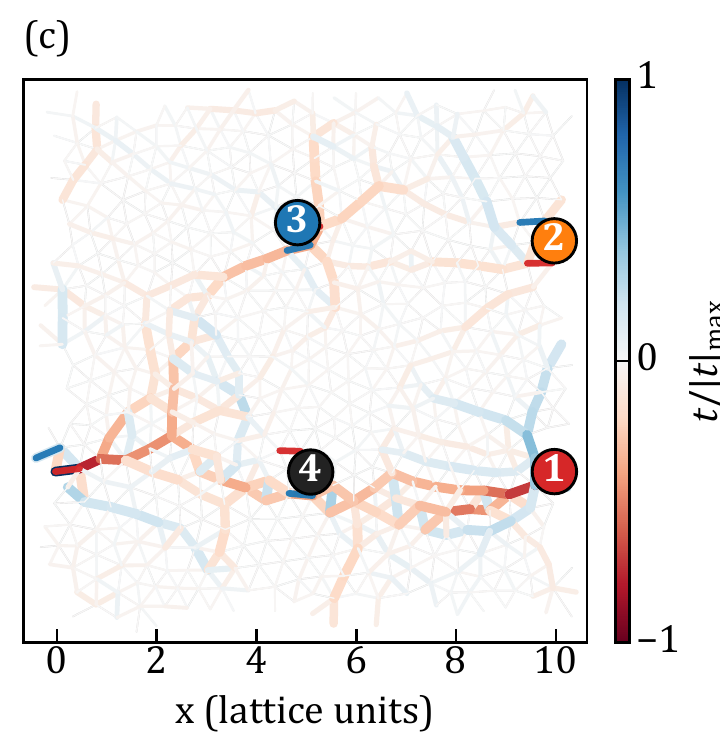
The physical pathway. Training rearranges the crosslink stiffnesses into connected force chains that carry the contact load to a far-side motor anchor.
Figure 4c · arXiv:2611.07112
Timing matters: the signal has to switch the motors before the 0.11-second contact ends. At physiological loads the trained wall does this easily; an untrained wall does not.
In simulations, the learned routing survives continuous enzymatic turnover of the wall, provided the tension-bearing crosslinks are preferentially protected from severing.
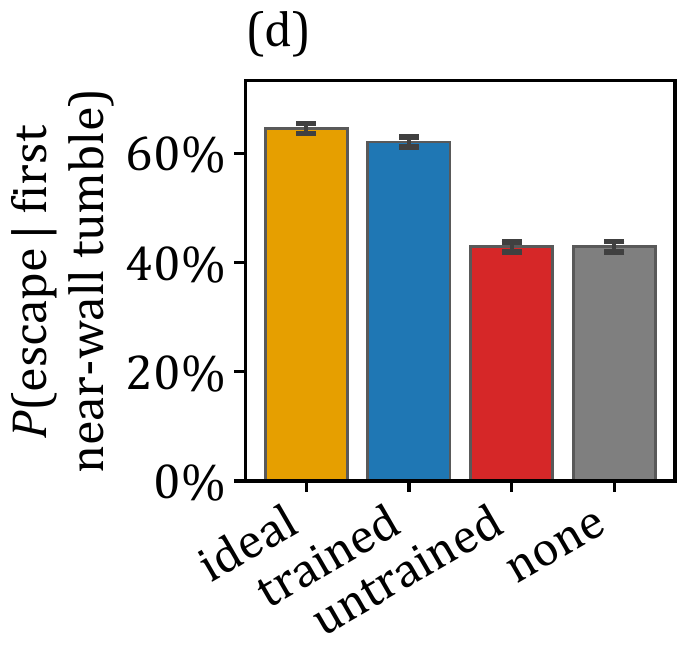
Behavior without a brain. On the first near-wall tumble, the trained wall escapes 62% of the time, against 43% for an untrained wall and 65% for an ideal controller.
Figure 6d · arXiv:2611.07112
Does learning create a need for sleep, even without biology?
Learning uses up a spring network’s capacity to learn. Repair brings that capacity back, and repair works better once the task is set aside.
We study a minimal physical learner: a spring network trained on a continual stream of tasks. Learning gradually uses up its ability to learn new ones, echoing the synaptic homeostasis hypothesis of sleep (Tononi & Cirelli 2006).
Learning pushes each bond’s share of the load toward a limit, where the bond has less influence on a new task: a mechanical analogue of sleep pressure (Borbély et al. 2016).
To impose an analogue of reversible quiescence, we turn off the task drive and suspend the learning rule after each task visit. Probed with small random forces, the quiet network lets each bond read its own load share from its mean elastic energy and adjust its stiffness to restore learning capacity. With the task on, task strain adds energy to the bonds in use and biases this repair toward weakening them.
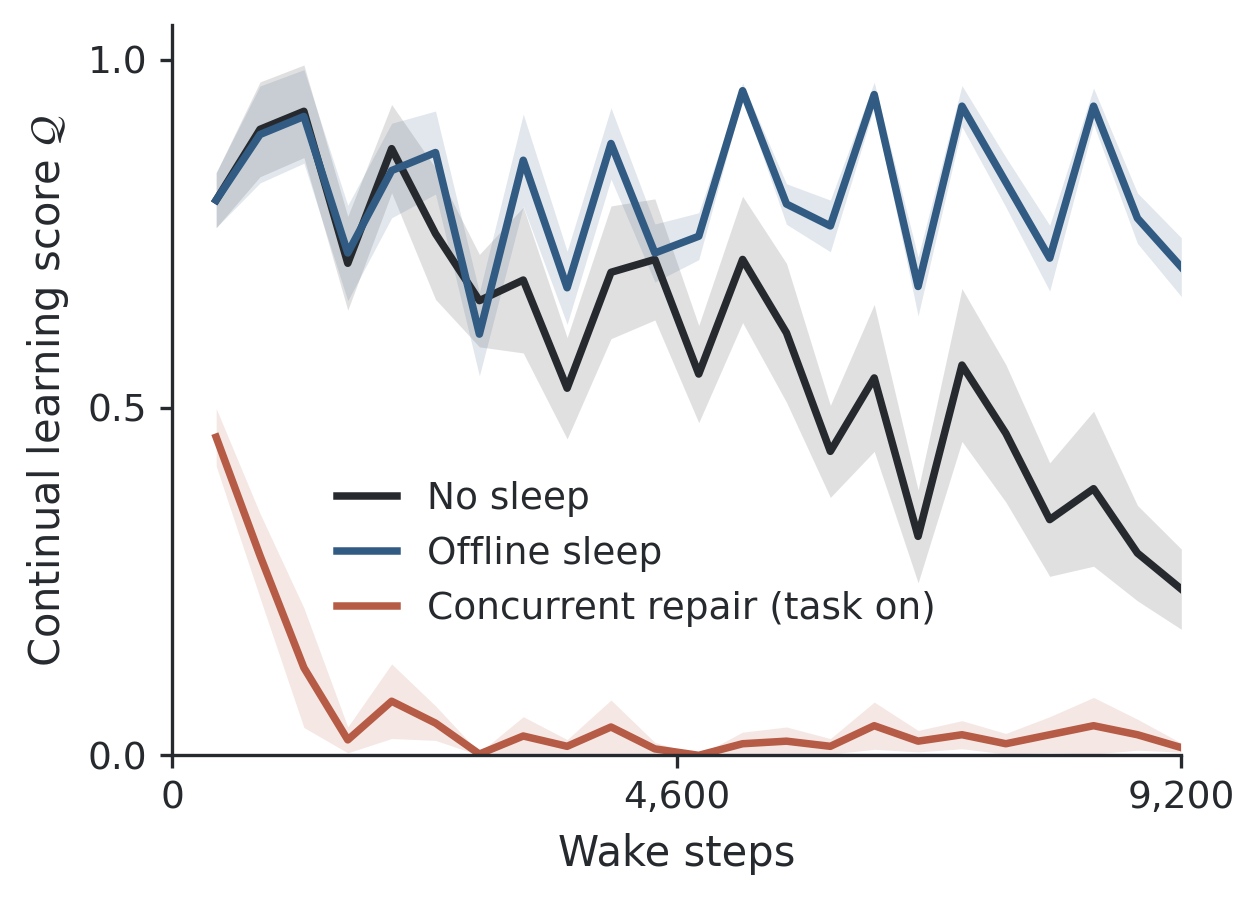
Why the repair has to be offline. Continual learning score over a stream of tasks, mean ± s.e.m. over 15 networks. Offline sleep keeps the score high, while without sleep the score declines. Repair run concurrently, with the task on, makes the score collapse.
Figure 4c · arXiv:2611.22070
Here an external supervisor schedules wake and repair. Whether that offline phase can arise on its own is the next project, Emergence of sleep–wake rhythms.
How do crypts form in an intestinal organoid?
Organoids are miniature intestines grown in the lab: a single stem cell can grow into one, complete with crypts, the pockets where stem cells live (Sato et al. 2009). With M. Blatchley, I am modeling how crypts form, using a three-dimensional vertex model of a spheroid in the extracellular matrix.
What role do cell shape and mechanical interactions play as crypts form?
How does the extracellular matrix affect the organoid’s shape and the formation of crypts?
How do interactions between cells and matrix shape tissue architecture in three dimensions?
Can a daily rhythm arise by itself?
This project follows Sleep without biology, with N. Pashine and J. M. Schwarz. There, an external supervisor decides when the offline phase happens.
Living systems make that switch themselves. They harvest and dissipate energy to sense errors (Lan et al. 2012), revise their own structure, and decide when to disengage from the environment.
The aim is to find the energetic conditions under which an offline phase emerges on its own, and how a demand for repair can couple to environmental energy cycles to produce a sleep–wake rhythm.
Full essays are gradually moving here.
Recent
Preprint · arXiv:2611.22070
With N. Pashine and J. M. Schwarz. Read the paper
Preprint · arXiv:2611.07112
With N. Chen and J. M. Schwarz. Read the paper
Poster · Boulder Summer School
Talk · APS March Meeting, Denver
Poster · MPI-PKS, Dresden
Older talks, teaching, and service are in my CV.
Photographs by Nada Elmeligy · @sedated_gaze
Select a photograph to view it in full.
About
My path began with an undergraduate degree in theoretical high-energy physics at Zewail City in Egypt. I started my PhD at Syracuse in experimental quantum computing, and in 2024 I joined the Jennifer Schwarz theory group and began working on the physics of learning in living and non-living matter.
Two commitments shape my vision. The first is to study nature on its own terms, rather than through the categories we expect it to fit—similar to how material-semiotic networks treat categories as outcomes of relations. The second is to make scientific ideas available across the economic, cultural, and linguistic divides that still decide who can read, contribute to, and benefit from science.
Outside the lab, I photograph, write, and occasionally paint.
Get in touch
nnelmeli@syr.eduIf you are curious about the work, want to collaborate, or are working to widen access to science, I would be glad to hear from you.
